AQUIFEX AEOLICUS VF5 · ORGANISM-SPECIFIC DESCRIPTION
How this system works in Aquifex
VF5 encodes NiFe-hydrogenase subunits, quinone-linked redox complexes, terminal oxidases and F0F1 ATP-synthase components. Experimental work has characterized Aquifex respiratory supercomplexes, including a sulfide-oxidizing, oxygen-reducing assembly. Electron-donor oxidation, quinone reduction, terminal electron transfer and ion coupling are distinct operations. An ion gradient across an intact membrane can drive ATP synthesis. The overview does not place every annotated subunit in one supercomplex or assert that all respiratory branches operate together under every growth condition.
31 proteins are assigned to this function in the 912-protein working reconstruction (Energy conservation and ATP synthesis).
The working reconstruction retains 912 proteins; 338 additional proteins remain undetermined. These are model selections, not a demonstrated viable minimum or individual VF5 knockout results. The 16 atlas hotspots and the reconstruction categories use different partitions.
Inspect the 912-protein inventory and model evidence →REFERENCE ORGANISM · AQUIFEX AEOLICUS VF5
Aquifex system diagram
51 selected annotated proteins · 6 functional modules
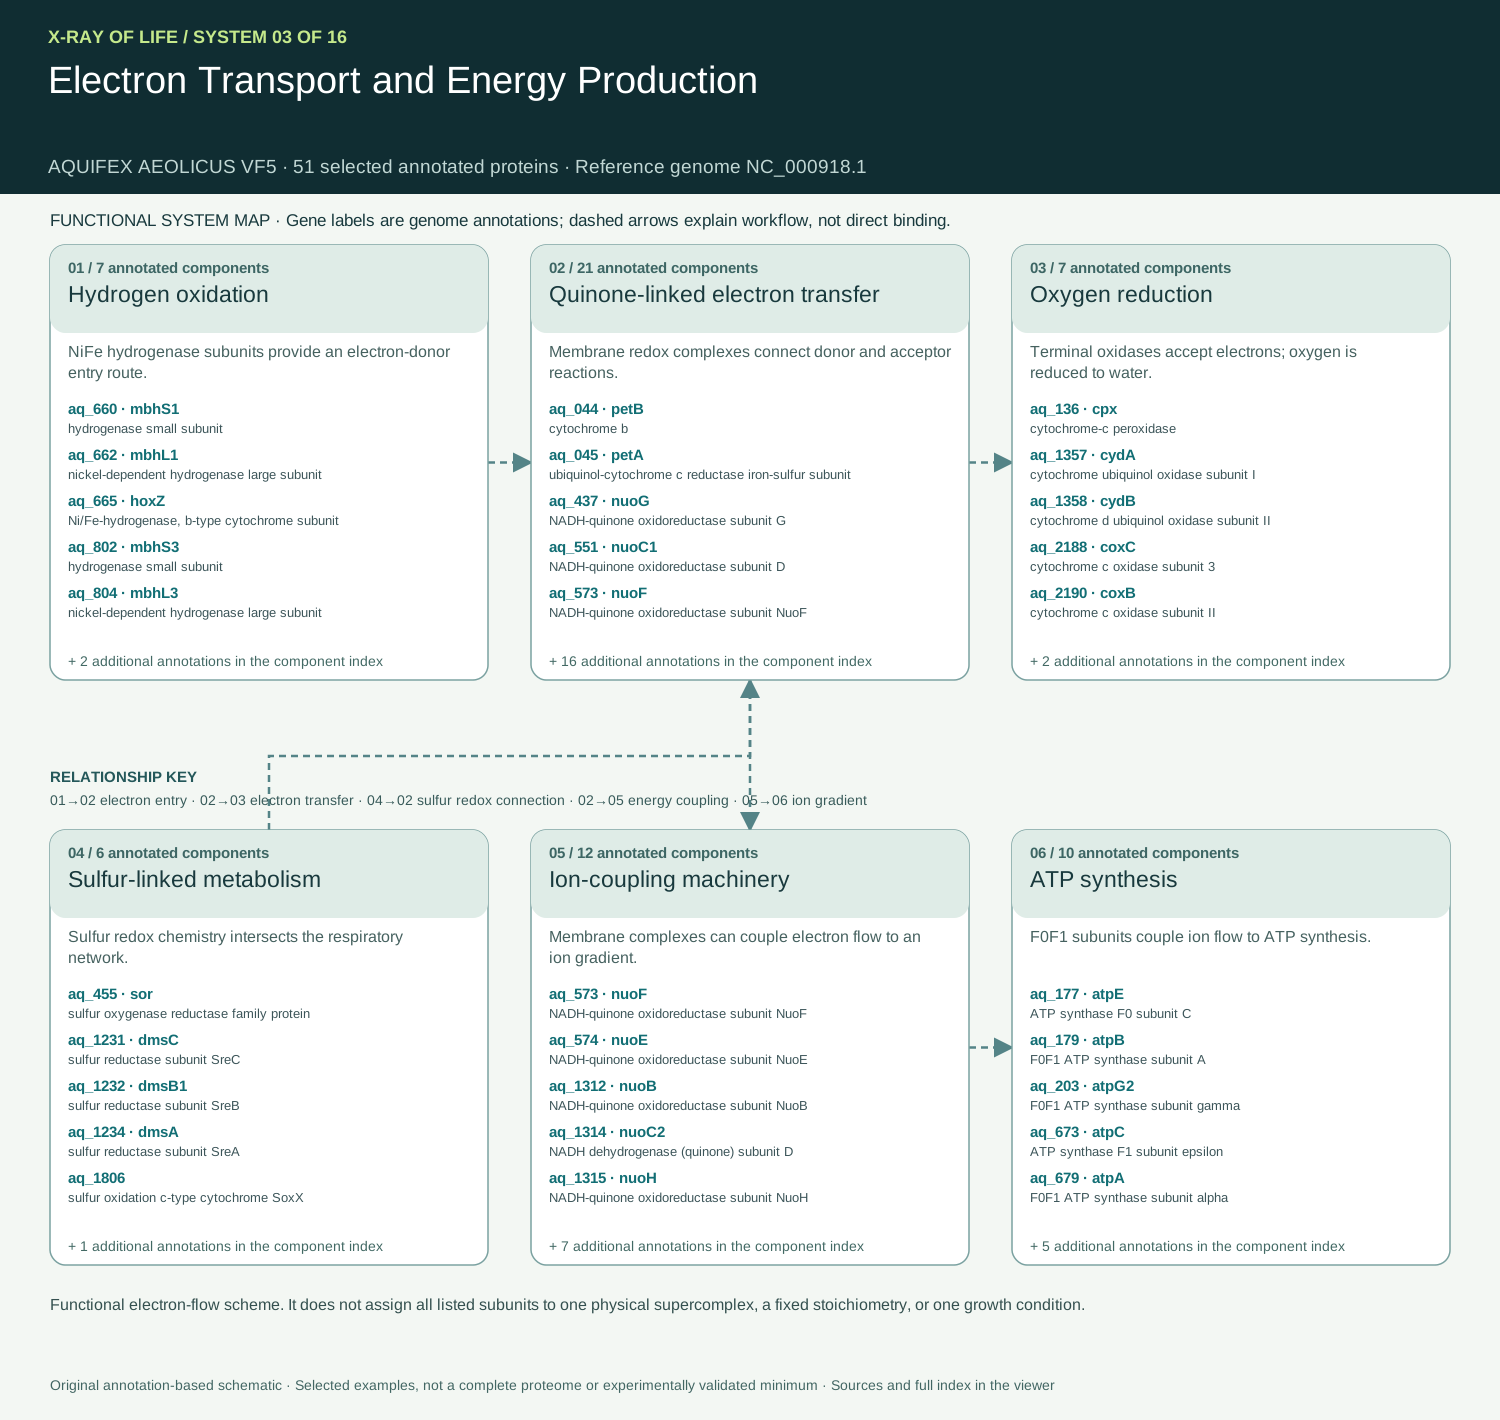 Open the full diagram and component evidence ↗
Electron-transfer chains couple inorganic donors to energy conservation. Click to read the full diagram and inspect the annotated protein records.
Original schematic from VF5 RefSeq annotations. Dashed arrows describe functional relationships; they are not measured protein interactions. Sources: Deckert et al. (1998), complete VF5 genome · Prunetti et al. (2010), purified Aquifex respiratory supercomplex · NCBI reference genome.
Functional electron-flow scheme. It does not assign all listed subunits to one physical supercomplex, a fixed stoichiometry, or one growth condition.
FUNCTION AND MECHANISM
How this system works
FOLLOW THE FLOW
Electron flow to conserved energy
Electron donor → electron-transfer chain → ion gradient → ATP synthase → ATP-dependent work
Electron Transport and Energy Production
Turning chemical energy into usable ATP
ATP is a molecule whose reactions help power much of the cell’s work.
A substance gives up electrons
Depending on the organism, this may be hydrogen or a food-derived molecule. A compatible electron acceptor is also needed; it is not always oxygen.
Move electrons through membrane proteins
Some steps use the released energy to move charged particles called ions across the membrane.
Build up an ion difference
More ions on one side, together with an electrical difference, store usable energy across the membrane.
Let ions return through ATP synthase
This molecular machine couples ion movement to joining ADP and phosphate to make ATP.
ATP supports cellular work
After ATP is used, ADP and phosphate can be used again to make ATP.
Read from top to bottom. Side-by-side panels show branches or supplies that come together; their labels explain the relationship. Detailed mechanisms and sources follow below.
Starting inputs: A compatible electron donor and acceptor, suitable membrane complexes, an ion-retaining membrane, ADP, and inorganic phosphate.
- Supply electrons: Oxidize a suitable donor and transfer electrons to the appropriate carriers.
- Transfer electrons toward an acceptor: Pass electrons through a compatible chain to a terminal acceptor. Energy-conserving steps couple this chemistry to ion movement; not every complex pumps ions.
- Build an electrochemical gradient: Accumulate a difference in ion concentration and electrical potential across the membrane while limiting uncontrolled leakage.
- Couple downhill ion flow to ATP synthesis: Ions moving through ATP synthase drive rotation and catalytic changes that produce ATP from ADP and inorganic phosphate.
- Use and replenish ATP: Cellular work consumes ATP. Metabolism restores the gradient and ATP pool as ADP and phosphate return to the cycle.
Usable outputs: ATP and membrane electrochemical gradients used by biosynthesis, transport, and maintenance.
This sequence describes respiratory chemiosmosis. Substrate-level phosphorylation is a parallel ATP-producing route. ATP synthase can run in reverse under suitable conditions, consuming ATP to pump ions.
Evidence for selected mechanisms
Structure of a bacterial ATP synthase
These papers examine the named mechanisms or networks. The numbered order is an explanatory overview; it is not an experimentally established history of cellular origins.
Starting with an electron donor and acceptor
An electron donor supplies electrons; an acceptor ultimately receives them. Hydrogen, reduced organic molecules, or sulfur compounds can play donor roles in appropriate organisms. Oxygen is one possible acceptor, but anaerobic cells use other chemical arrangements. A hypothetical cell needs a compatible donor–acceptor pair and enzymes able to connect the reactions.
Conserving energy across a membrane
Electron-transfer reactions can be coupled to movement of protons or other ions. This creates an electrochemical difference between the two sides of the membrane. The membrane must limit uncontrolled ion leakage, while proteins provide regulated pathways. Not every electron-transfer step pumps ions, and the coupling architecture varies among organisms.
How ATP synthase works
In a proton-driven ATP synthase, protons move through the membrane portion and drive rotation. The rotor changes the shape of catalytic sites in the soluble portion, enabling ATP formation from ADP and inorganic phosphate. A stationary support prevents the whole assembly from rotating together. Under suitable conditions the enzyme can run in reverse, consuming ATP to move ions.
Matching energy supply to use
Biosynthesis, transport, molecular repair, and chromosome management consume energy. Energy carriers and electron carriers must therefore be regenerated continuously. A cell may also produce ATP through substrate-level phosphorylation, in which a chemical group-transfer reaction is coupled directly to ATP formation. The selected routes must fit the cell’s actual environment and carbon metabolism.
A closer look at the evidence
Cryo-electron microscopy resolved a bacterial ATP synthase in different rotational states, supporting the structural explanation of membrane-coupled ATP production.1
Follow the consequence
A damaged membrane can allow ions to leak back without passing through ATP synthase. Electron transport may continue, yet less of its energy is conserved for ATP production.
Component families in this system (12)
- Cytochrome bc1 complex III
- Cytochrome c oxidase complex
- NADH dehydrogenase Complex I-related
- ATP Synthase Complex V
- Hydrogen Oxidation
- Sulfur Metabolism basic
- Succinate dehydrogenase and hydrogenase
- Oxidoreductase for anaerobic metabolism
- Ferredoxin-based electron transport
- Sulfur metabolism pathway enzymes
- NAD+ biosynthesis via Aspartate
- Alternative electron transport
FUNCTIONALLY INTEGRATED
What it depends on, and why
A functional dependency means that one process supplies material, energy, machinery, or suitable conditions to another. It does not necessarily mean that two proteins physically touch.
| Other system | Relationship | Why the connection matters |
|---|---|---|
| 01 · Carbon metabolism | Receives from this system | ATP and reducing equivalents support energy-requiring carbon assimilation and precursor production. The exact coupling depends on the chosen fixation pathway. |
| 02 · Cofactors | Receives from this system | ATP and reducing power drive cofactor synthesis and regeneration. |
| 02 · Cofactors | Provides to this system | Flavin, NAD, and other cofactors participate in electron-transfer reactions. |
| 07 · Lipids & membrane | Provides to this system | A sufficiently ion-tight membrane supports electrochemical gradients and houses respiratory and ATP-synthase complexes. |
| 16 · Metal clusters | Provides to this system | Selected electron-transfer proteins require Fe–S clusters or other metal centers to function. |
| 05 · Nucleotides | Receives from this system | Energy investment supports nucleotide synthesis and phosphorylation. |
| 06 · Amino acids | Receives from this system | ATP and reducing power drive energy-requiring amino acid biosynthesis. |
| 07 · Lipids & membrane | Receives from this system | ATP and reducing power support membrane-component synthesis. |
| 08 · DNA processing | Receives from this system | ATP powers selected helicase, ligase, and chromosome-management reactions. |
| 09 · RNA & translation | Receives from this system | ATP supports tRNA charging and GTP supports major translation steps; energy supply must replenish these currencies. |
| 10 · Signaling & regulation | Receives from this system | ATP supports phosphorylation and other energy-dependent regulatory processes. |
| 11 · Transport | Receives from this system | ATP or ion gradients drive active transport, depending on transporter type. |
| 12 · Quality control | Receives from this system | Many chaperones, remodeling enzymes, and proteolytic systems consume ATP. Not every QC reaction requires ATP. |
| 14 · Homeostasis | Receives from this system | Energy supply supports pumps and other active maintenance processes. |
| 15 · Stress response | Receives from this system | Energy supply supports many protective, repair, and protein-turnover responses. |
REASON & SCIENCE LIBRARY · ORGANIZING QUESTIONS
Library basis for this article
The library connects respiratory electron flow, a membrane gradient and ATP-producing machinery. This article uses that dependency as its organizing question: how is released energy captured as useful work? The organism-specific account must identify actual donors, acceptors and coupling components rather than transpose the complete mammalian respiratory chain into a bacterial membrane.L
FUNCTIONAL ORGANIZATION · AUTHOR’S FRAMEWORK
Hallmarks of design
Energy production illustrates the following organizational features in the supplied papers. These descriptions identify biological functions; interpreting their origin as design is the author’s comparative argument.H1, H2
Membrane energy conservation depends on a maintained electrochemical gradient.
Electron transfer and ion movement must couple to ATP production in the selected respiratory chain.
Electron donors, acceptors, membrane integrity and cellular work must be compatible.
Origin hurdles and abductive assessment · Assessment method · All 40 hallmarks. Biological evidence: the mechanism, accession records and scientific references on this page.
SOURCE-BASED SYNTHESIS
The origin problem in brief
How could a membrane, energy gradient, and energy-converting machinery first work together?
- Capture environmental energy in a form that can drive useful chemistry.
- Couple an ion gradient, a suitable membrane, and ATP-producing machinery.
- Coordinate electron carriers, metal cofactors, and energy supply with cellular demand.
Source notes and how the count is used
Energy problems span several source categories. No separate atlas-aligned total is assigned.
Numbers reproduce the source’s reported section totals. They are not a new count of unique questions or an independent assessment of which issues remain scientifically unresolved. Overlapping lists are not added together.
Source passages: X-ray of Life, Volume II, Chapter 4; §§14.1–14.2, pp. 179–220; 752–754; X-ray of Life, Volume III, §§15.4–15.5, pp. 560–578; The Cell: An Unsolved Mystery, Chapter 9, pp. 174–189.
The overview follows the cell-specific scope of Forty Hallmarks of Design in the Cell: later eukaryotic machinery, specialized immune systems, and model-specific numerical probabilities are not treated as universal first-cell requirements.
ORIGINS
What needs to be explained
An origins explanation must connect available chemistry to a system that can persist, reproduce useful functions, and pass them to descendants. Explaining how a modern system works and explaining how its predecessors arose are different tasks. Simpler catalysts, environmental assistance, and alternative chemistries must be evaluated rather than assuming that the complete modern machinery appeared at once.
Scope of the question
Aerobic respiratory complexes and anaerobic alternatives are not all assumed to coexist. The origin of cellular energy conversion must be assessed for a specified chemical environment.
Major hurdles to investigate
These are requirements to test in proposed scenarios. Their importance depends on the environment and on which intermediate system is proposed.
Available energy
Identify a sustained source of chemical disequilibrium rather than a single energetic event.
Coupling
Channel energy into useful synthesis instead of allowing it to dissipate as heat.
Boundary properties
Combine nutrient permeability with sufficient retention of ions and metabolites.
Catalyst organization
Arrange electron carriers and catalysts so that forward transfer outcompetes unproductive reactions.
Transition to autonomy
Explain how environmental energy coupling became inherited cellular machinery.
EXPERIMENTAL PROGRESS
What has been demonstrated, and what it leaves open
Hydrogen-driven mineral chemistry has reproduced selected reactions related to carbon and energy metabolism. Such results inform possible energy sources before enzymes; they do not establish the origin of an ion-tight membrane, a rotary ATP synthase, or their coordinated operation.2
Condensed origin challenges
- Capture environmental energy in a form that can drive useful chemistry.
- Couple an ion gradient, a suitable membrane, and ATP-producing machinery.
- Coordinate electron carriers, metal cofactors, and energy supply with cellular demand.
Three condensed themes from the source passages above; they are not the complete numbered catalogue.
The integration test
Experiments that connect precursor chemistry across molecular classes help test compatibility.3 A strong next test for this system would combine its relevant chemical steps with continued material supply, energy use, retention, and reproduction under an explicitly specified environmental sequence. The open questions above are research questions, not claims that every intermediate is impossible.
Engineered minimal cells help reveal present cellular dependencies, but their construction starts from existing biological machinery and growth conditions. They therefore answer a different question from a prebiotic synthesis experiment.4
Explore prebiotic synthesis challengesTERMS IN PLAIN LANGUAGE
Glossary
- electron donor / acceptor
- The donor gives up electrons (e.g. H₂ or NADH); the acceptor at the end of the chain takes them (e.g. O₂ or a sulfur compound).
- electron-transfer chain
- A series of membrane proteins and carriers that pass electrons step by step and use the released energy to pump ions.
- ferredoxin
- A small iron–sulfur protein that carries electrons between enzymes.
- quinone
- A small fat-soluble carrier that moves electrons (and protons) within the membrane.
- cytochrome
- A protein containing a heme iron group that carries electrons; complex bc₁ and cytochrome oxidase are examples.
- hydrogenase
- An enzyme that takes electrons from hydrogen gas (H₂) or releases them as H₂.
- Complex I (NADH dehydrogenase)
- The membrane complex that takes electrons from NADH and pumps protons.
- ion gradient
- More ions (such as H⁺ or Na⁺) on one side of the membrane than the other, storing energy like water behind a dam.
- ATP synthase
- A rotary membrane machine that lets ions flow back in and uses that flow to make ATP from ADP and phosphate.
- chemiosmosis
- Making ATP using an ion gradient across a membrane, rather than directly in a chemical reaction.
- substrate-level phosphorylation
- Making ATP directly in a metabolic reaction, without an ion gradient.
- ADP + Pi
- Adenosine diphosphate and inorganic phosphate: the parts that ATP synthase joins to make ATP.
- enzyme
- A molecule, usually a protein, that speeds up a chemical reaction without being consumed by it.
- ATP
- Adenosine triphosphate: a molecule whose chemical reactions can be coupled to many energy-requiring cellular processes. It is continually used and regenerated.
- ion
- An atom or molecule with a net electrical charge.
- gradient
- A difference across space, such as a difference in ion concentration or electrical potential across a membrane.
Related library threads
Your Inner Locomotive Revealed · The electron transport chain · The irreducibly complex ATP Synthase nanomachine, amazing evidence of design
The author’s library essays and research compilations provide context and arguments. Biological mechanisms should be assessed through the scientific references; the design inference is a separate, revisable assessment.
SCIENTIFIC LITERATURE
Scientific papers
Linked superscript numbers in the text lead to the papers below, numbered in order of first citation on this page. Each entry links to the publisher and bibliographic record; open full text is included where available. These studies support the specified mechanisms or experiments, not every possible origin scenario.
Guo H, Suzuki T, Rubinstein JL. (2019). Structure of a bacterial ATP synthase. Elife, 8, e43128.
Preiner M, Igarashi K, Muchowska KB, Yu M, Varma SJ, Kleinermanns K, Nobu MK, Kamagata Y, Tüysüz H, Moran J, Martin WF. (2020). A hydrogen-dependent geochemical analogue of primordial carbon and energy metabolism. Nat Ecol Evol, 4, 534-542.
Patel BH, Percivalle C, Ritson DJ, Duffy CD, Sutherland JD. (2015). Common origins of RNA, protein and lipid precursors in a cyanosulfidic protometabolism. Nat Chem, 7, 301-307.
Hutchison CA, Chuang RY, Noskov VN, Assad-Garcia N, Deerinck TJ, Ellisman MH, Gill J, Kannan K, Karas BJ, Ma L, Pelletier JF, Qi ZQ, Richter RA, Strychalski EA, Sun L, Suzuki Y, Tsvetanova B, Wise KS, Smith HO, Glass JI, Merryman C, Gibson DG, Venter JC. (2016). Design and synthesis of a minimal bacterial genome. Science, 351, aad6253.
Further scientific reading
7 additional papers. Each title links to its article or bibliographic record.
Search and filter this system’s reference list →